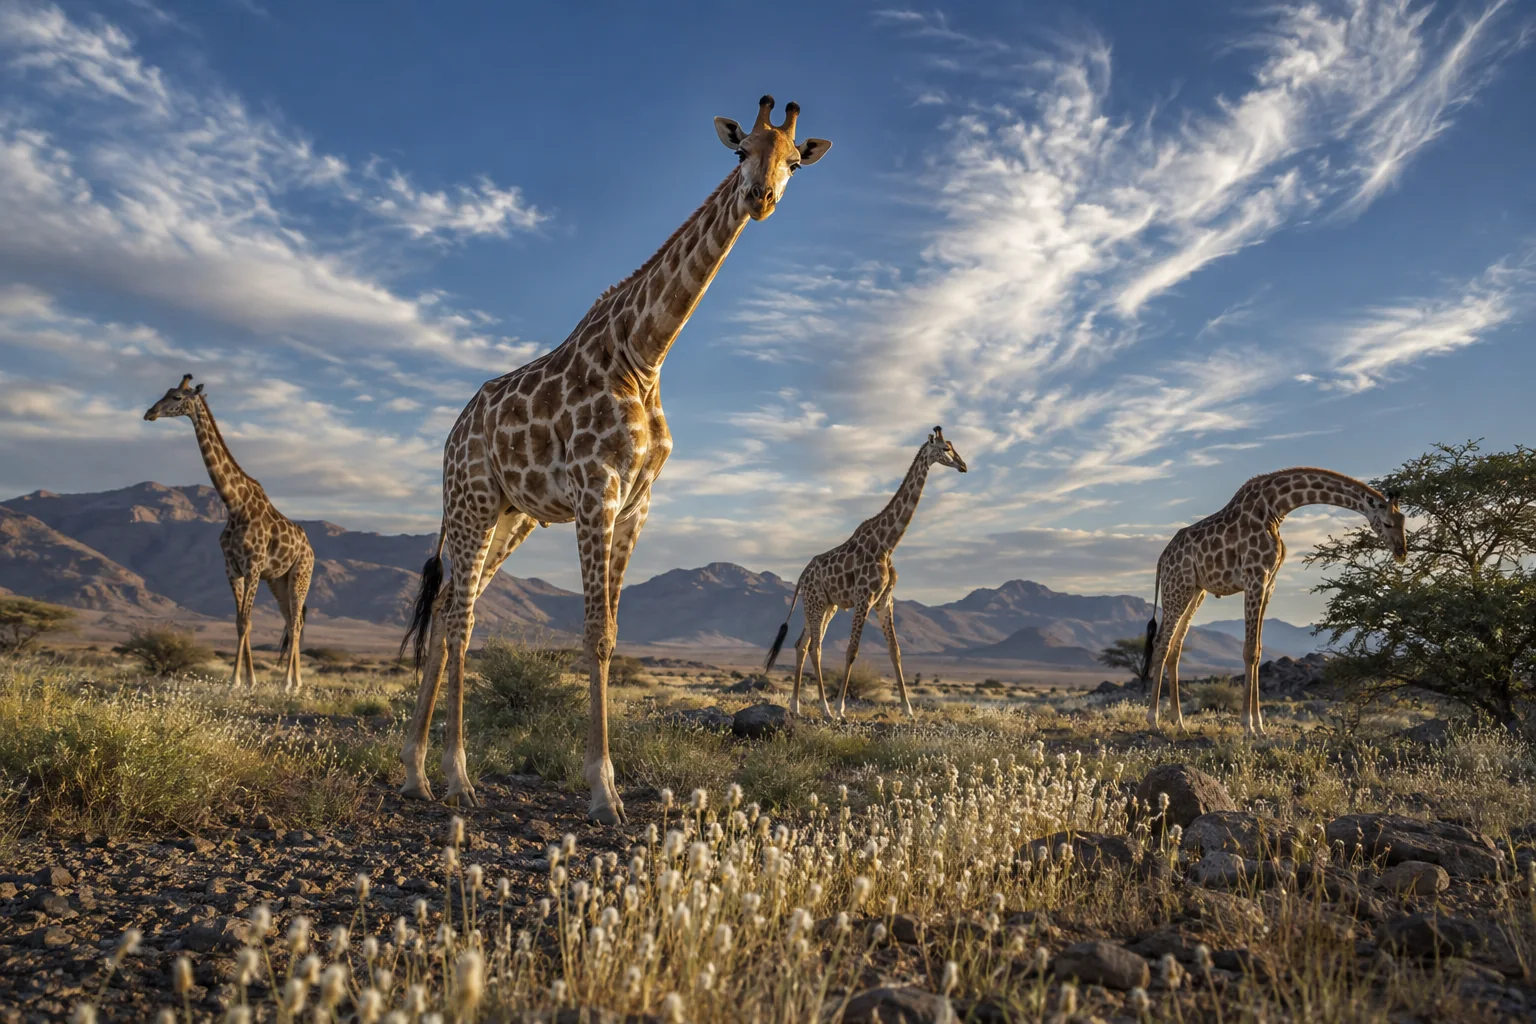
Where scientists study giraffes can change their understanding of what threatens a population. Look mainly inside protected areas and adult survival may seem dependable, with the fate of calves supplying much of the variation. Extend the study into neighbouring landscapes and the adults can become the unstable part of the system.
That was the central discovery of a 2016 study by Derek E. Lee and colleagues. The team compared giraffe survival and reproduction across five parts of Tanzania's Tarangire ecosystem, then set those results alongside published estimates from elsewhere in Africa. Adult female survival varied far more across the local management landscape than it did in the mostly protected populations represented in the broader literature.
The result is about more than the importance of keeping adult giraffes alive. It shows how a plausible ecological rule can depend on which landscapes supply the evidence.
Why calves were expected to vary more
Giraffes live long lives and reproduce slowly. In a population where most adult females survive from year to year, a bad season may show up especially clearly among calves. Young animals are vulnerable, and their survival can fluctuate while the breeding adults persist.
This creates two different questions. First, how strongly would population growth respond if a survival rate changed? Second, which rates actually vary enough to explain observed differences between populations?
An adult female's survival may have a large potential effect on future population growth because she can reproduce repeatedly. Yet if adult survival is almost the same everywhere being compared, it cannot explain much of the difference among those places. More variable calf survival or reproduction may explain more, even if changing each by the same proportional amount would have a smaller effect.
The paper tested that distinction. It asked whether adult survival was relatively constant and juvenile survival more variable, and whether the rates with the largest potential influence were also the ones accounting for differences in population growth.
Looking across management boundaries
The researchers worked in Tarangire and Lake Manyara national parks, Manyara Ranch Conservancy, and two game controlled areas. Together, these places spanned contrasting levels of wildlife protection, settlement, cultivation and livestock use.
They photographed giraffes on repeated road surveys from 2012 through 2014. Individual coat patterns allowed them to recognise the same animals again. The analysis followed 860 adult females and 449 calves.
Repeat encounters are essential to this kind of study. A giraffe absent from one survey may be alive but overlooked, so the researchers used capture–recapture models to estimate survival while allowing detection to be imperfect. Photographic identification also allowed them to measure the appearance of new calves relative to the adult female population.
The resulting survival estimates were apparent survival: they could not completely separate death from permanent movement out of the sampled population. The authors acknowledged that limitation, which can pull survival estimates and projected growth downwards. Their strongest use of the data was comparing rates across areas, rather than treating each projected growth rate as an exact forecast.
The models then combined age-specific survival and reproduction into a female population life cycle. Calves surviving their first year progressed through subadult stages; survivors eventually entered the breeding population. Because some age-specific rates were difficult to estimate directly, the researchers used an age pattern derived from known-age females to interpolate survival during the subadult years.
The pattern depended on the comparison
Across all five Tarangire areas, adult survival was about as variable, in proportional terms, as calf survival and reproduction. That was already a departure from the expected pattern of stable adult survival and more variable early life.
But when the researchers restricted the regional comparison to the two national parks and Manyara Ranch, adult survival became much less variable. The familiar pattern returned.
The continental comparison told a similar story. Published adult survival estimates from mostly protected populations averaged about 0.90 per year and varied comparatively little. Calf survival and reproduction showed larger proportional variation.
These are not contradictory findings. They describe different sets of places. The mixed local landscape included management settings in which adult females disappeared at much higher rates than in the better-protected areas. The protected-area comparison excluded much of that variation.
A useful way to read the result is as a warning about the sampling frame. Evidence collected in secure habitats can correctly describe those habitats while leaving out precisely the pressure that matters in less-secure ones.
What drove the differences in population growth?
The population models made the consequence visible. Adult survival had the largest potential influence on growth in all the populations analysed. More unusually, differences in adult survival also supplied most of the modelled explanation for why growth differed across the five regional sites.
The authors attributed 81% of the regional variation apportioned among demographic components to adult survival, compared with 7% to calf survival and 12% to fecundity. These percentages are model decomposition results. They do not mean that 81% of giraffes died from one threat, or that 81% of a conservation budget should automatically go to one intervention.
Figure 4 of the paper makes the comparison particularly clear. In the regional analysis, the large negative contributions in the two game controlled areas came predominantly from adult survival. The corresponding bars for calf survival and reproduction were much smaller.
Across the continental comparison, the attribution was more distributed: adult survival still contributed most, but calf survival and fecundity accounted for larger shares than in the local analysis. Which life stage explains population differences therefore depends partly on how those populations differ in the first place.
Protection was associated with survival, not experimentally isolated
The researchers investigated environmental and management explanations for the pattern. Adult survival was positively associated with their measure of anti-poaching effort, and they considered illegal hunting a likely major cause of the lower rates in less-protected areas.
That interpretation fits the contrast they observed, but the study did not randomly assign protection or directly determine the cause of every disappearance. Management, livestock presence, human activity and predator conditions varied together. Competing models involving lion density and management also received support.
These correlations matter when interpreting the conservation message. The results support concern about adult mortality in less-protected landscapes; they do not prove that one particular enforcement action would reproduce a specified survival increase. Nor do they isolate livestock grazing as the cause of poor performance. Manyara Ranch, which combined wildlife conservation with grazing, belonged to the group with relatively stable adult survival.
Survival estimates also retained the permanent-emigration limitation. A missing female could represent a death or a move outside the monitored system. More detailed movement information would help resolve that ambiguity.
Following the animals beyond the boundary
A subsequent study by Lee and Douglas T. Bolger used movement information from the same broader research programme to investigate connections among these five areas. It classified the two national parks and Manyara Ranch as demographic sources and the game controlled areas as sinks.
That later analysis adds context rather than independent confirmation: it used overlapping encounter records and the demographic estimates developed here. Its contribution was to show why a local count can conceal dependence on arriving animals, and why differences in survival need to be considered within a connected system.
Together, the studies suggest a practical monitoring question. If a protected population looks stable, what happens to recognisable giraffes using its surrounding landscape? The answer can reveal losses that a park-only study would miss.
A broader view of what stability means
The paper does not overturn the observation that young giraffes can be highly vulnerable. It shows why that observation cannot become a universal assumption about the main driver of population change.
Adult survival looked stable when comparisons stayed largely within protected areas. Once the researchers included a stronger range of human pressures, that stability weakened, and adult survival dominated differences in the population models.
Conservation evidence needs to span the places animals actually use. Otherwise, a study can describe survival inside a boundary accurately while giving an incomplete account of the population that crosses it.
Sources
Derek E. Lee, Monica L. Bond, Bernard M. Kissui, Yustina A. Kiwango and Douglas T. Bolger (2016). “Spatial variation in giraffe demography: a test of 2 paradigms.” Journal of Mammalogy 97:1015–1025. Full paper.
Derek E. Lee and Douglas T. Bolger (2017). “Movements and source–sink dynamics of a Masai giraffe metapopulation.” Population Ecology 59:157–168. Connected movement analysis.