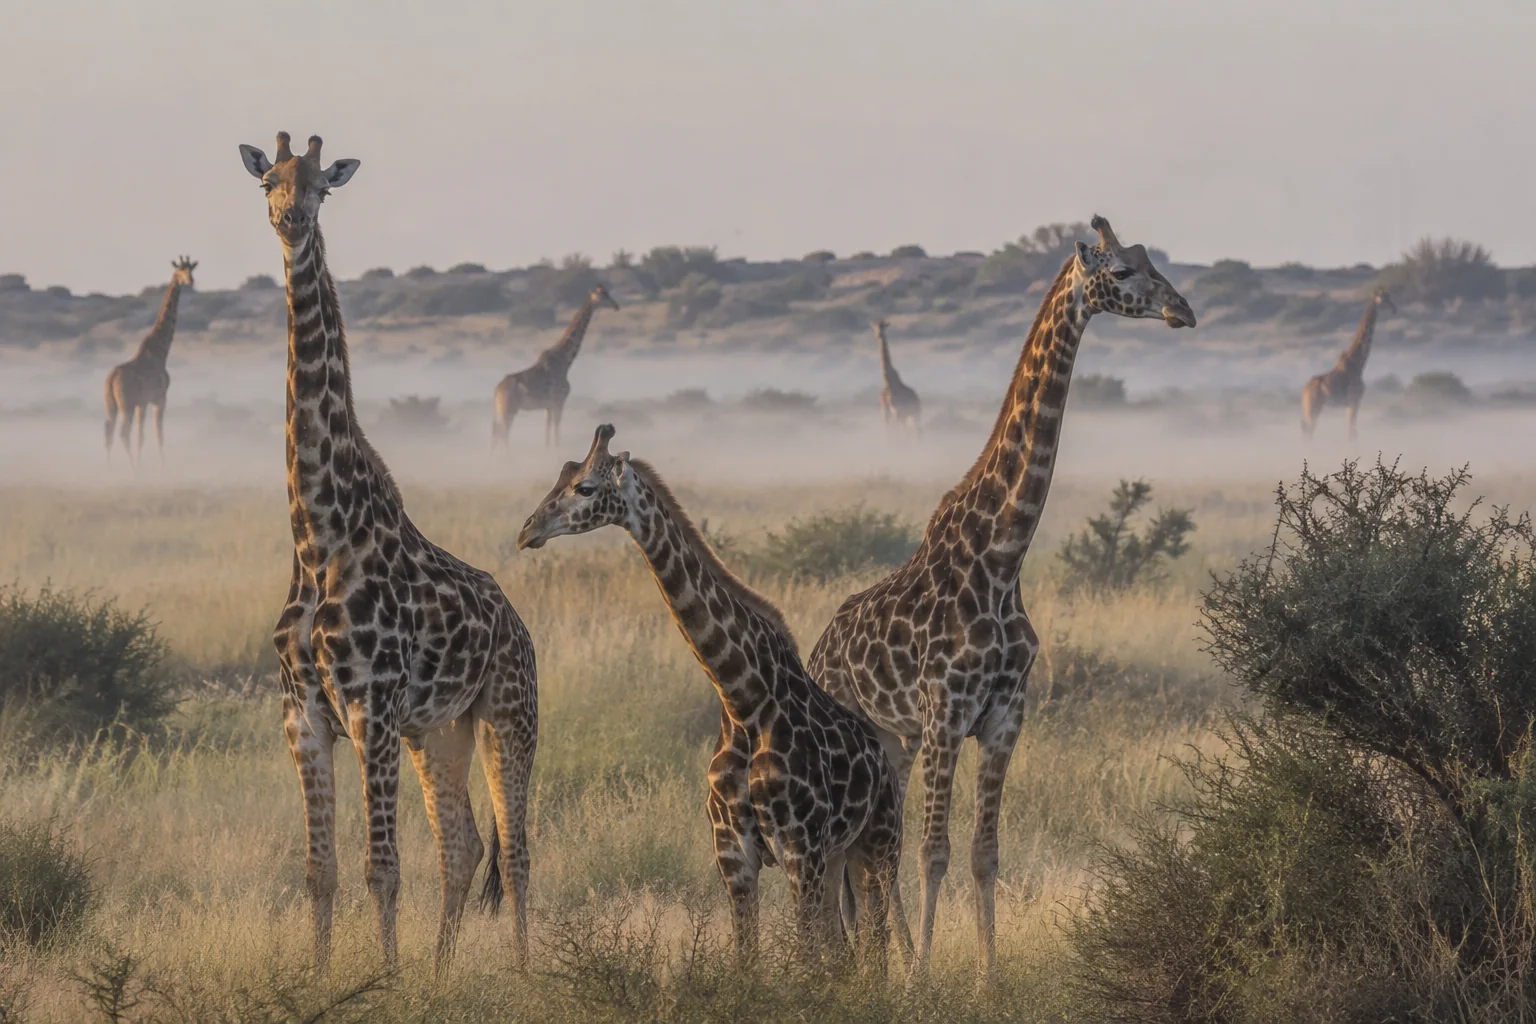
Two giraffes lost every five years might sound like an occasional event. For a small population, however, those deaths can remove breeding animals faster than the population can replace their contribution. A modelling study of Kordofan giraffes in Cameroon’s Bénoué National Park found that such infrequent adult losses could sharply worsen an already precarious simulated future.
Starting with 40 giraffes, the researchers compared thousands of possible population histories. Their baseline model reached extinction in 78.6% of runs over 100 years. Removing one adult female and one adult male every five years raised that proportion to 98.1%.
Those percentages were model outputs, not a measured probability that Bénoué’s giraffes would disappear on a particular timetable. Kane Colston and colleagues designed the 2023 study to compare threats and interventions despite substantial gaps in local demographic knowledge. Its most useful result was the contrast between scenarios: protecting adults, especially females, mattered far more than simply assuming that a large park had room for more animals.
Simulating individual lives
A population viability analysis follows a population through imagined futures under specified rules. In this study, the VORTEX program represented individual giraffes that could survive, die and reproduce. Random variation meant that the same starting conditions did not always produce the same ending.
This matters when numbers are small. An average expectation of births and deaths can conceal very different realized outcomes. A few unfavourable years, or an unfortunate sequence of losses among breeding animals, can have consequences that a smooth average growth curve misses.
The researchers ran each scenario 5,000 times for 100 years. They defined extinction as the point when only one sex remained. Thus, the model’s extinction endpoint was loss of the possibility of reproduction within the isolated population, not necessarily the death of its last animal.
The baseline began with 40 giraffes, drawing on the population information available to the team. It assumed a stable age distribution and treated the park population as closed, with no routine exchange with neighbouring areas. That last choice reflected uncertainty about movement; it was not field evidence that the park was isolated.
Many biological inputs also had to come from elsewhere. Survival estimates were drawn from Tanzanian populations, breeding schedules from giraffe studies, and a drought scenario from a combination of regional rainfall data and assumed effects on survival and reproduction. The authors selected adult mortality estimates intended to exclude poaching, so that they could add adult removals separately and examine their effect.
The resulting baseline was therefore a constructed reference population. It was neither a complete reconstruction of Bénoué’s recent history nor a direct measurement of its current vital rates.
Why the occasional losses accumulated
The poaching scenarios removed fixed numbers of adults at specified intervals. In the least frequent removal scenario, the model lost one adult of each sex every five years. That pair represents a different biological burden as a population shrinks: the removal remains two animals even when fewer animals are available to replace them.
Compared with the baseline, this scenario raised the proportion of runs reaching extinction within the century by 19.5 percentage points, from 78.6% to 98.1%. Annual removal of one adult female and one adult male produced extinction in all simulated runs, with a mean time to extinction of approximately 15 years.
| Model scenario | Extinction within 100 years |
|---|---|
| Baseline, no explicit poaching | 78.6% |
| One adult female and one adult male removed every five years | 98.1% |
| One adult female and one adult male removed every year | 100% |
| Two adult females removed every year | 100% |
The last two scenarios reached the same century-scale endpoint, but their timing differed. Removing two adult females annually produced a mean time to extinction of approximately 11 years, compared with 15 years for one adult of each sex. The number lost was the same. Their reproductive roles made the difference.
The model allowed a male to breed with multiple females, and not every adult male belonged to the breeding pool. Losing a female removed one of the animals directly producing calves; losing a male did not necessarily reduce the number of females that could breed. This is a consequence of the specified mating system, rather than a claim that males never limit population persistence.
The simulations did not establish Bénoué’s actual poaching rate. Nor did they measure the effectiveness of a patrol programme. They showed the consequences of stipulated adult losses, supporting the authors’ priority of preventing such losses while collecting better local information.
Adding animals helped, but their sex mattered
The researchers also simulated supplementation: adding adult giraffes to the population. They tested both the number introduced and the balance of females and males.
Adding 24 females in the first year reduced the modelled century-scale extinction probability to 40.9%. Adding 24 males reduced it only slightly, to 77.6%, close to the 78.6% baseline. An equal addition of 12 females and 12 males produced an intermediate result of 56.7%.
These comparisons illuminate the same reproductive bottleneck from the opposite direction. If breeding females are scarce, adding females can expand the population’s capacity to produce calves. A large addition of males does not necessarily do so when enough males are already available for mating.
Even the stronger supplementation scenarios did not guarantee sustained recovery. In the simulation that added 12 females and 12 males in both year 1 and year 11, extinction probability remained 34% over the century. The population could remain larger than the baseline for decades while still declining over the longer term. A conspicuous rise after an introduction was therefore insufficient evidence of a self-sustaining population.
The authors also separated a modelled benefit from the practical case for moving animals. They argued that translocation would be unjustified while the threats affecting the receiving population remained inadequately controlled. Availability of suitable giraffes, the risks and costs of moving them, and their fate after release were not solved by a favourable simulation.
Supplementation could also represent immigration from neighbouring populations. That interpretation made connectivity a central question: protecting movement routes might allow animals to join the population without a managed transfer. The model did not demonstrate that such immigration currently occurred or would be sufficient.
Space was not the only limiting resource
The study varied carrying capacity, the number of giraffes the modelled habitat could support. Its baseline capacity was much higher than the starting population, making habitat space relatively plentiful within the model’s assumptions.
Increasing that ceiling alone had little effect on persistence. This is understandable: creating theoretical room for more animals does not immediately repair an unfavourable balance of births and deaths in a population far below the ceiling. By contrast, reducing capacity could worsen the simulated outcome.
That asymmetry is not evidence that habitat restoration is unimportant. It depends partly on how the model represents habitat. Here, carrying capacity acted through a ceiling on abundance; it did not fully represent the ways deteriorating food or movement opportunities could change reproduction and survival before the ceiling was reached. The authors also noted that truncating abundance above capacity could exaggerate mortality compared with a real population that dispersed or adjusted its reproduction.
The useful interpretation is narrower: an intervention that improves one limiting factor may achieve little if another factor continues to drive decline. The model supported considering survival, habitat and additions together, while avoiding a universal ranking detached from local conditions.
The most useful uncertainties were biological
The team varied uncertain inputs to identify which ones most affected its simulated growth rate. Four accounted for 87.6% of the variation examined: the proportion of adult females breeding, the sex ratio at birth, adult female mortality and subadult mortality.
These sensitivity results point toward specific field measurements. How often do females produce calves? How many females and young giraffes survive from one year to the next? Does the observed adult sex ratio reflect the sexes at birth or different survival afterwards?
A more precise headcount alone would not answer those questions. Within the tested range, changing the initial population size had little influence on the simulated growth rate. That does not mean abundance is unimportant, or that a larger population has the same extinction risk. It means that the model’s direction of growth was controlled chiefly by the rules governing births and survival.
The authors also cautioned that some parameter combinations explored in sensitivity analysis were biologically implausible. Its broad ranges were a way to examine dependence on assumptions, not a catalogue of equally likely giraffe populations.
Field photographs supply the next step
A separate photographic assessment of Bénoué, by Connor Parks and colleagues, illustrates both the foundation and the limits of the available field evidence. It identified 26 giraffes in the park and estimated approximately 27, while acknowledging restricted coverage and a collection period spanning several years. No identified individual was shared with the other surveyed area.
The modelling study’s starting 40 and the photographic paper’s estimate 27 should not be mistaken for consecutive censuses demonstrating further decline. The modelling work drew on earlier population information from the same research setting; these are related evidence streams and differing estimates, not independent confirmation of a forecast. Our photo-census account explains that distinction and the remaining uncertainty about exchange.
Following those recognizable giraffes over time could improve the very survival and reproductive inputs that the model found influential. Establishing movement between areas would test its assumption of isolation. Recording actual losses would show whether the hypothetical removal scenarios resemble the pressures the population faces.
The study makes a strong case for treating even occasional adult deaths as consequential. It also explains why the response needs evidence about individual lives. When few giraffes remain, knowing how many are present is only the beginning of understanding whether they can persist.
Sources
Colston, Kane P. J.; Johnson, Caspian L.; Nyugha, Denis; Mengamenya Goué, Achile; and Penny, Samuel G. (2023). “Viability analysis of Kordofan giraffe (Giraffa camelopardalis antiquorum) in a protected area in Cameroon.” African Journal of Ecology, 61, 929–944. Paper and DOI. Full paper.
Parks, Connor; Penny, Samuel; Mengamenya Goue, Achile; Nyugha, Denis; Pauline, Tiwa T.; Vannier, Xavier; and Johnson, Caspian (2023, online publication). “Preliminary population estimate of Kordofan giraffe (Giraffa camelopardalis antiquorum) in two areas of the Benoué complex, Cameroon.” African Journal of Ecology, e13249. Paper and DOI.